MDCAT · Biology (PMDC curriculum) · Unit 6: Enzymes
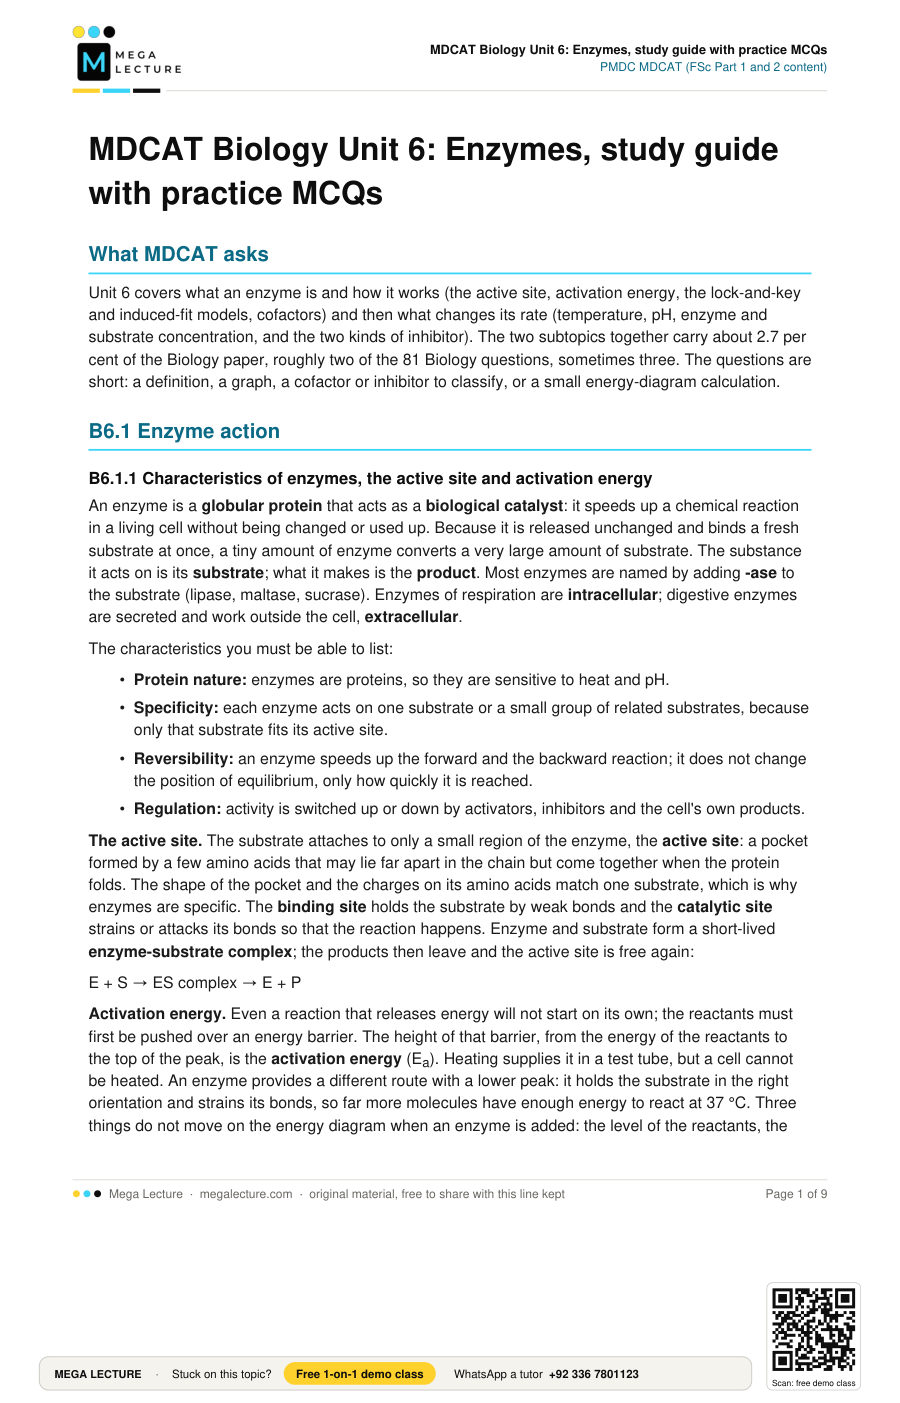
MDCAT Biology Unit 6: Enzymes, study guide with practice MCQs
Need more than one subject? All-notes pass: unlimited downloads of every note for a year: unlimited downloads of every note on the site, PKR 999 a year. All packs and courses.
Opens inside this page. Prefer your own PDF app? Open the PDF.
Check yourself
5 quick questions on MDCAT Biology
Tap an answer to see if you are right, and why. Free, no sign-up.
Start the free testWas this note useful?
Full text of MDCAT Biology Unit 6: Enzymes, study guide with practice MCQs
What MDCAT asks
Unit 6 covers what an enzyme is and how it works (the active site, activation energy, the lock-and-key and induced-fit models, cofactors) and then what changes its rate (temperature, pH, enzyme and substrate concentration, and the two kinds of inhibitor). The two subtopics together carry about 2.7 per cent of the Biology paper, roughly two of the 81 Biology questions, sometimes three. The questions are short: a definition, a graph, a cofactor or inhibitor to classify, or a small energy-diagram calculation.
B6.1 Enzyme action
B6.1.1 Characteristics of enzymes, the active site and activation energy
An enzyme is a globular protein that acts as a biological catalyst: it speeds up a chemical reaction in a living cell without being changed or used up. Because it is released unchanged and binds a fresh substrate at once, a tiny amount of enzyme converts a very large amount of substrate. The substance it acts on is its substrate; what it makes is the product. Most enzymes are named by adding -ase to the substrate (lipase, maltase, sucrase). Enzymes of respiration are intracellular; digestive enzymes are secreted and work outside the cell, extracellular.
The characteristics you must be able to list:
- Protein nature: enzymes are proteins, so they are sensitive to heat and pH.
- Specificity: each enzyme acts on one substrate or a small group of related substrates, because only that substrate fits its active site.
- Reversibility: an enzyme speeds up the forward and the backward reaction; it does not change the position of equilibrium, only how quickly it is reached.
- Regulation: activity is switched up or down by activators, inhibitors and the cell's own products.
The active site. The substrate attaches to only a small region of the enzyme, the active site: a pocket formed by a few amino acids that may lie far apart in the chain but come together when the protein folds. The shape of the pocket and the charges on its amino acids match one substrate, which is why enzymes are specific. The binding site holds the substrate by weak bonds and the catalytic site strains or attacks its bonds so that the reaction happens. Enzyme and substrate form a short-lived enzyme-substrate complex; the products then leave and the active site is free again:
E + S → ES complex → E + P
Activation energy. Even a reaction that releases energy will not start on its own; the reactants must first be pushed over an energy barrier. The height of that barrier, from the energy of the reactants to the top of the peak, is the activation energy (Ea). Heating supplies it in a test tube, but a cell cannot be heated. An enzyme provides a different route with a lower peak: it holds the substrate in the right orientation and strains its bonds, so far more molecules have enough energy to react at 37 °C. Three things do not move on the energy diagram when an enzyme is added: the level of the reactants, the level of the products and therefore the overall energy change. Only the peak comes down.
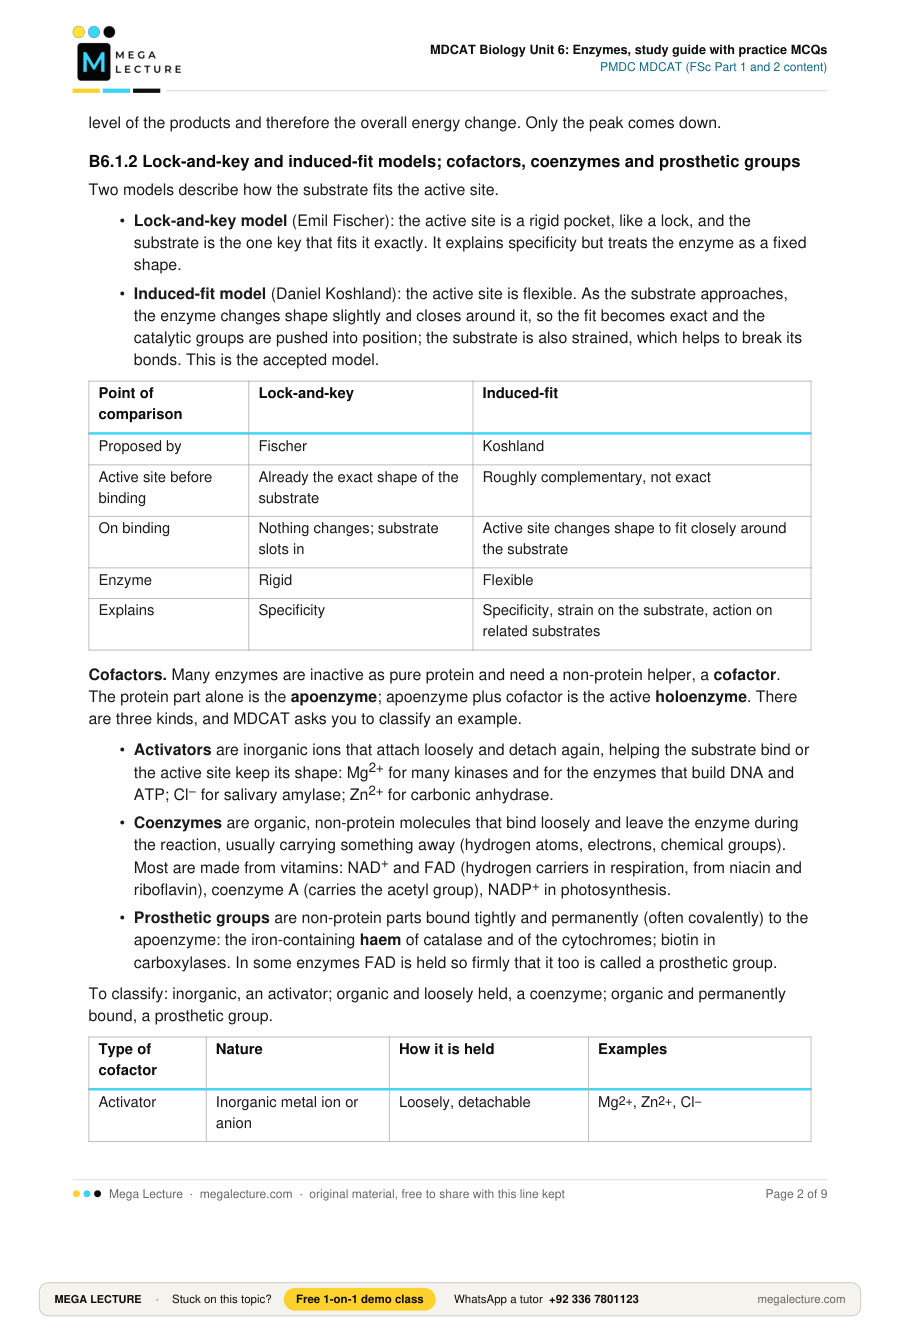
B6.1.2 Lock-and-key and induced-fit models; cofactors, coenzymes and prosthetic groups
Two models describe how the substrate fits the active site.
- Lock-and-key model (Emil Fischer): the active site is a rigid pocket, like a lock, and the substrate is the one key that fits it exactly. It explains specificity but treats the enzyme as a fixed shape.
- Induced-fit model (Daniel Koshland): the active site is flexible. As the substrate approaches, the enzyme changes shape slightly and closes around it, so the fit becomes exact and the catalytic groups are pushed into position; the substrate is also strained, which helps to break its bonds. This is the accepted model.
| Point of comparison | Lock-and-key | Induced-fit |
|---|---|---|
| Proposed by | Fischer | Koshland |
| Active site before binding | Already the exact shape of the substrate | Roughly complementary, not exact |
| On binding | Nothing changes; substrate slots in | Active site changes shape to fit closely around the substrate |
| Enzyme | Rigid | Flexible |
| Explains | Specificity | Specificity, strain on the substrate, action on related substrates |
Cofactors. Many enzymes are inactive as pure protein and need a non-protein helper, a cofactor. The protein part alone is the apoenzyme; apoenzyme plus cofactor is the active holoenzyme. There are three kinds, and MDCAT asks you to classify an example.
- Activators are inorganic ions that attach loosely and detach again, helping the substrate bind or the active site keep its shape: Mg2+ for many kinases and for the enzymes that build DNA and ATP; Cl− for salivary amylase; Zn2+ for carbonic anhydrase.
- Coenzymes are organic, non-protein molecules that bind loosely and leave the enzyme during the reaction, usually carrying something away (hydrogen atoms, electrons, chemical groups). Most are made from vitamins: NAD+ and FAD (hydrogen carriers in respiration, from niacin and riboflavin), coenzyme A (carries the acetyl group), NADP+ in photosynthesis.
- Prosthetic groups are non-protein parts bound tightly and permanently (often covalently) to the apoenzyme: the iron-containing haem of catalase and of the cytochromes; biotin in carboxylases. In some enzymes FAD is held so firmly that it too is called a prosthetic group.
To classify: inorganic, an activator; organic and loosely held, a coenzyme; organic and permanently bound, a prosthetic group.
| Type of cofactor | Nature | How it is held | Examples |
|---|---|---|---|
| Activator | Inorganic metal ion or anion | Loosely, detachable | Mg2+, Zn2+, Cl− |
| Coenzyme | Organic, often vitamin-derived | Loosely, leaves during the reaction | NAD+, NADP+, FAD, coenzyme A |
| Prosthetic group | Organic or metal-containing group | Tightly, usually covalently, permanent | Haem in catalase and cytochromes, biotin |
MDCAT trap: the enzyme changes the peak, not the ends
Wrong options in this unit give the enzyme a power it does not have.
- An enzyme does not supply energy to the reaction; it lowers the activation energy by offering an easier route.
- It does not change the energy of the reactants, the energy of the products or the difference between them. "Makes the reaction release more energy" or "raises the energy of the products" is wrong.
- It does not change the position of equilibrium; it only makes equilibrium arrive sooner.
- It is not used up. Reject "consumed" or "becomes part of the product".
- Apoenzyme is the protein alone; holoenzyme is protein plus cofactor.
Worked example: reading an energy diagram
Question. Reactants sit at 60 kJ mol−1 and products at 25 kJ mol−1. The peak is at 140 kJ mol−1 without the enzyme and at 90 kJ mol−1 with it. Find (a) the activation energy with and without the enzyme, (b) how much the enzyme lowers it, (c) the overall energy change in each case.
Step 1. Activation energy is peak minus reactants. Without enzyme: 140 − 60 = 80 kJ mol−1. With enzyme: 90 − 60 = 30 kJ mol−1.
Step 2. The enzyme lowers the activation energy by 80 − 30 = 50 kJ mol−1.
Step 3. Overall energy change is products minus reactants: 25 − 60 = −35 kJ mol−1, with or without the enzyme, because those two levels do not move.
Answer. (a) 80 and 30; (b) lowered by 50; (c) −35 kJ mol−1 in both cases.
B6.2 Factors and inhibition
B6.2.1 Temperature, pH, enzyme concentration and substrate concentration
The rate of an enzyme-catalysed reaction (product formed per unit time) depends on how often substrate molecules collide with free active sites and on whether the active site has kept its shape.
Temperature. Warming gives enzyme and substrate molecules more kinetic energy, so they collide more often and more collisions carry the activation energy. For many enzymes the rate roughly doubles for every 10 °C rise (Q10 about 2) up to the optimum temperature, about 37 °C for most human enzymes. Beyond the optimum the extra vibration breaks the weak bonds (hydrogen, ionic, hydrophobic) that hold the tertiary structure; the active site loses its shape and the substrate no longer fits. The enzyme is denatured and the rate falls steeply, reaching zero at roughly 60 °C. Heat denaturation is usually permanent: cooling does not restore the shape. The peptide bonds survive; the fold is lost. Cold is different. Near 0 °C the molecules move too slowly to collide, so the enzyme is inactive, and it works again as soon as it is warmed; this is why freezing preserves food.
pH. Each enzyme has an optimum pH at which the charges on the amino acids of the active site are exactly those needed to bind the substrate. Moving away from it in either direction adds or removes H+ ions, altering the charges on the R groups, breaking ionic and hydrogen bonds and changing the shape of the active site, so the rate falls. The graph is a narrow bell with its peak at the optimum. A small shift is reversible; an extreme pH denatures the enzyme.
| Enzyme | Where it works | Optimum pH |
|---|---|---|
| Pepsin | Stomach | About 2 |
| Salivary amylase | Mouth | About 6.8 |
| Most intracellular enzymes | Cytoplasm | About 7 to 7.4 |
| Trypsin | Small intestine | About 8 |
| Pancreatic lipase | Small intestine | About 9 |
Enzyme concentration. If substrate is in excess, every added enzyme molecule finds substrate at once, so the rate is directly proportional to enzyme concentration: a straight line through the origin, which flattens only if substrate or a cofactor runs short.
Substrate concentration. With the enzyme amount fixed, adding substrate at first raises the rate almost in proportion, because more active sites are filled each second. The increase then slows and the rate reaches a plateau, the maximum rate (Vmax). Now every active site is occupied all the time, the enzyme is saturated, and extra substrate has nowhere to bind; only more enzyme can raise the rate further.
B6.2.2 Competitive and non-competitive inhibition
An inhibitor lowers the rate by interfering with the enzyme. Inhibition is normal in cells, where it controls pathways, and many drugs and poisons are enzyme inhibitors. Inhibitors are classified by where they bind (competitive or non-competitive) and by how firmly (reversible or irreversible).
Competitive inhibition. The inhibitor has a shape similar to the substrate, so it fits into the active site and sits there without reacting; while it is there the substrate cannot bind. Substrate and inhibitor compete for the same site, so raising the substrate concentration pushes the inhibitor out and the rate climbs back. At a high enough substrate concentration the normal Vmax is still reached. Examples: malonate competes with succinate for succinate dehydrogenase in the Krebs cycle; sulphonamide drugs block a bacterial enzyme by mimicking its substrate.
Non-competitive inhibition. The inhibitor does not resemble the substrate and binds at a different place on the enzyme, away from the active site. Binding there distorts the protein, so the active site changes shape and no longer works, even though nothing is sitting in it. Because inhibitor and substrate are not competing for the same site, adding more substrate does not help: the fraction of enzyme molecules disabled stays the same and Vmax is lowered. Examples usually quoted: cyanide, which binds the iron of cytochrome oxidase; heavy-metal ions such as Hg2+ and Ag+, which react with the sulphur of cysteine residues.
Reversible and irreversible. A reversible inhibitor binds by weak bonds and comes off again, so the enzyme recovers when it is removed; most competitive inhibitors are reversible. An irreversible inhibitor forms a strong covalent bond and destroys the enzyme's activity for good: cyanide, heavy-metal ions, nerve gases.
Feedback inhibition. Cells use reversible non-competitive inhibition to regulate pathways. When the end product of a pathway builds up, it binds to a site on the first enzyme (the allosteric site) and switches it off; when the product is used up it leaves and the pathway restarts. This is end-product or feedback inhibition, and the enzyme is an allosteric enzyme.
| Point of comparison | Competitive inhibitor | Non-competitive inhibitor |
|---|---|---|
| Shape | Resembles the substrate | Need not resemble the substrate |
| Binds at | The active site | A site other than the active site (allosteric site) |
| Effect on active site | Blocks it physically | Changes its shape from a distance |
| Adding more substrate | Overcomes the inhibition | Does not overcome it |
| Maximum rate (Vmax) | Still reached, at a higher substrate concentration | Lowered |
| Usual reversibility | Reversible | Reversible (feedback inhibition) or irreversible (cyanide, Hg2+) |
| Examples | Malonate on succinate dehydrogenase; sulphonamides | Cyanide on cytochrome oxidase; heavy-metal ions; end products of pathways |
MDCAT trap: cold inactivates, heat denatures
Students lose this mark by writing that a low temperature "denatures" an enzyme.
- Inactivation by cold: molecules move too slowly to collide, the active site is intact, the effect is reversible on warming.
- Denaturation by heat, extreme pH or heavy metals: weak bonds holding the tertiary structure break, the active site loses its shape, the effect is normally permanent. Cooling a boiled enzyme does not revive it.
- Do not say the enzyme is "killed": an enzyme is a molecule, not a living thing. The word is denatured.
- "More substrate restores the rate" or "resembles the substrate" means competitive; "binds away from the active site" or "maximum rate is lowered" means non-competitive.
Worked example: telling the inhibitors apart from the numbers
Question. An enzyme gives a maximum rate of 40 units at high substrate concentration. With inhibitor X the rate falls sharply at low substrate, but when the substrate concentration is raised far enough it climbs back to 40 units. With inhibitor Y instead, the rate falls and never rises above 20 units however much substrate is added. Classify X and Y.
Step 1. With X the original Vmax of 40 units is still reachable; the enzyme just needs more substrate. Substrate can displace X, so the two compete for the active site. X is a competitive inhibitor and must resemble the substrate.
Step 2. With Y the maximum is halved and no amount of substrate recovers it. Substrate cannot displace Y, so Y is not in the active site; it binds elsewhere and distorts the active site, putting half the enzyme molecules out of action. Y is non-competitive.
Answer. X is competitive (same Vmax, overcome by substrate); Y is non-competitive (lower Vmax, not overcome by substrate).
Practice MCQs
Question 1. Which statement correctly describes what an enzyme does to a chemical reaction?
- A. It lowers the activation energy and is recovered unchanged at the end.
- B. It raises the energy of the products so that the reaction releases more energy.
- C. It is used up in forming the product.
- D. It shifts the equilibrium towards the products.
Question 2. On an energy diagram the reactants are at 30 kJ mol−1 and the products at 10 kJ mol−1. The peak is at 80 kJ mol−1 without the enzyme and at 55 kJ mol−1 with it. Which statement is correct?
- A. The activation energy with the enzyme is 20 kJ mol−1.
- B. The overall energy change is −20 kJ mol−1 both with and without the enzyme.
- C. The enzyme lowers the activation energy by 50 kJ mol−1.
- D. With the enzyme the products are raised to 35 kJ mol−1.
Question 3. As a substrate approaches an enzyme, the active site alters its shape slightly and closes around the substrate so that the fit becomes exact. This observation supports the:
- A. lock-and-key model of Fischer
- B. theory of feedback inhibition
- C. concept of the apoenzyme
- D. induced-fit model of Koshland
Question 4. Catalase contains an iron-containing haem group that is permanently and tightly bound to the protein and is essential for its activity. The haem group is best classified as a:
- A. activator
- B. coenzyme
- C. prosthetic group
- D. apoenzyme
Question 5. A purified enzyme shows no activity. When Mg2+ is added, full activity returns; when the Mg2+ is removed again by dialysis, activity is lost once more. Which conclusion is correct?
- A. Mg2+ is a coenzyme made from a vitamin.
- B. The purified protein was the apoenzyme and Mg2+ is a detachable activator.
- C. Mg2+ is a prosthetic group covalently bound to the enzyme.
- D. Purification denatured the enzyme and Mg2+ refolded it.
Question 6. The optimum pH of pepsin is about:
- A. 2
- B. 6.8
- C. 7.4
- D. 9
Question 7. With a fixed amount of enzyme, the rate of reaction rises as substrate concentration increases and then levels off at a constant maximum. The rate levels off because:
- A. the high substrate concentration denatures the enzyme
- B. the product formed acts as a competitive inhibitor
- C. every active site is occupied, so the enzyme is saturated
- D. the substrate molecules begin to bind to each other
Question 8. One sample of salivary amylase is kept at 0 °C for an hour and a second at 80 °C. Both are then brought to 37 °C and mixed with starch. What will be observed?
- A. Both samples digest starch normally.
- B. Neither sample digests starch, because both were denatured.
- C. Only the 80 °C sample digests starch, because heat activates enzymes.
- D. Only the 0 °C sample digests starch, because cold inactivation is reversible but heat denaturation is not.
Question 9. Which statement is true of a competitive inhibitor but not of a non-competitive inhibitor?
- A. Its effect can be overcome by raising the substrate concentration.
- B. It lowers the maximum rate of the reaction.
- C. It binds at a site other than the active site.
- D. It always binds to the enzyme by covalent bonds.
Question 10. Malonate slows the conversion of succinate to fumarate by succinate dehydrogenase. When the concentration of succinate is raised, the rate returns almost to normal. Which conclusion follows?
- A. Malonate binds covalently and irreversibly to the enzyme.
- B. Malonate changes the shape of the active site by binding at an allosteric site.
- C. Malonate denatures the enzyme at high concentration.
- D. Malonate resembles succinate and competes with it for the active site.
1. A. An enzyme lowers the activation energy and is released unchanged; it does not alter the product energy, is not consumed and does not move the equilibrium.
2. B. The overall change is products minus reactants, 10 − 30 = −20 kJ mol−1, and the enzyme does not alter it. With the enzyme the activation energy is 55 − 30 = 25, lowered from 50 by 25, not 50.
3. D. A change in the shape of the active site on binding is the induced-fit model of Koshland; the lock-and-key model treats the site as rigid.
4. C. A non-protein group bound tightly and permanently to the enzyme is a prosthetic group; activators and coenzymes are loosely held.
5. B. Activity lost on purification and restored by a loosely held inorganic ion shows that the protein alone is the apoenzyme and Mg2+ is an activator. An inorganic ion is not a coenzyme, and a detachable one is not a prosthetic group.
6. A. Pepsin works in the acid of the stomach and has an optimum pH of about 2. Salivary amylase is about 6.8 and pancreatic lipase about 9.
7. C. At the plateau all active sites are occupied all the time (saturation); only more enzyme can raise the rate further.
8. D. Cold only inactivates an enzyme and the effect is reversed on warming; 80 °C is far above the optimum and denatures amylase permanently.
9. A. A competitive inhibitor occupies the active site, so extra substrate displaces it and the normal maximum is still reached. B and C describe a non-competitive inhibitor.
10. D. Inhibition overcome by more substrate means inhibitor and substrate compete for the same site: malonate is a competitive inhibitor that mimics succinate. Irreversible, allosteric or denaturing inhibition would not be reversed by substrate.
Before the test: 12 facts to recite
- Enzymes are globular proteins that act as biological catalysts: they speed up reactions, are unchanged at the end and are needed in tiny amounts.
- Activation energy = energy of the peak − energy of the reactants. An enzyme lowers the peak only; reactant level, product level and overall energy change do not move.
- The active site is a small pocket of a few amino acids with a binding site and a catalytic site; its shape and charge give the enzyme its specificity.
- Lock-and-key (Fischer): rigid active site, exact fit. Induced-fit (Koshland, accepted): the active site changes shape as the substrate binds.
- Holoenzyme (active) = apoenzyme (protein) + cofactor (non-protein).
- Activator: detachable inorganic ion (Mg2+, Zn2+, Cl−). Coenzyme: loosely bound organic molecule, often from a vitamin (NAD+, FAD, coenzyme A). Prosthetic group: tightly, permanently bound (haem).
- Rate roughly doubles per 10 °C rise up to the optimum (about 37 °C for human enzymes); above it the enzyme is denatured, permanently. Cold only inactivates, reversibly.
- Optimum pH: pepsin about 2, salivary amylase about 6.8, trypsin about 8, pancreatic lipase about 9. pH acts by changing the charges on the active site.
- With excess substrate, rate is directly proportional to enzyme concentration: a straight line through the origin.
- With fixed enzyme, rate rises with substrate concentration and then plateaus at Vmax when all active sites are occupied (saturation).
- Competitive inhibitor: resembles the substrate, binds at the active site, overcome by more substrate, Vmax unchanged (malonate, sulphonamides).
- Non-competitive inhibitor: binds away from the active site and changes its shape, not overcome by more substrate, Vmax lowered (cyanide, Hg2+). Feedback inhibition: a pathway's end product switches off an early enzyme.
